BPTFbromodomain PHD finger transcription factor
Autism Reports / Total Reports
9 / 11Rare Variants / Common Variants
42 / 0Aliases
-Associated Syndromes
-Chromosome Band
17q24.2Associated Disorders
-Relevance to Autism
Missense variants in the BPTF gene have been identified in ASD probands from the MSSNG cohort, the SPARK cohort, the Autism Sequencing Consortium, and most recently in a cohort of 75 Turkish patients diagnosed with ASD (Yuen et al., 2017; Zhou et al., 2022; Fu et al., 2022; Kayhan et al., 2026). De novo loss-of-function variants in this gene have been reported in ASD probands from the REACH cohort and a Spanish ASD cohort, as well as in an individual with autism from a ethnically diverse pediatric patient population (Ji et al., 2019; Antaki et al., 2022; Blzquez et al., 2025). ASD has also been reported in a subset of individuals with NEDDFL (2/10 in Stankiewicz et al., 2017, and 3/26 individuals in Glinton et al., 2021).
Molecular Function
This gene was identified by the reactivity of its encoded protein to a monoclonal antibody prepared against brain homogenates from patients with Alzheimer's disease. Analysis of the original protein (fetal Alz-50 reactive clone 1, or FAC1), identified as an 810 aa protein containing a DNA-binding domain and a zinc finger motif, suggested it might play a role in the regulation of transcription. High levels of FAC1 were detected in fetal brain and in patients with neurodegenerative diseases. The protein encoded by this gene is actually much larger than originally thought, and it also contains a C-terminal bromodomain characteristic of proteins that regulate transcription during proliferation. The encoded protein is highly similar to the largest subunit of the Drosophila NURF (nucleosome remodeling factor) complex. In Drosophila, the NURF complex, which catalyzes nucleosome sliding on DNA and interacts with sequence-specific transcription factors, is necessary for the chromatin remodeling
External Links
SFARI Genomic Platforms
Reports related to BPTF (11 Reports)
| # | Type | Title | Author, Year | Autism Report | Associated Disorders |
|---|---|---|---|---|---|
| 1 | Support | Whole genome sequencing resource identifies 18 new candidate genes for autism spectrum disorder | C Yuen RK et al. (2017) | Yes | - |
| 2 | Support | - | Paweà â Stankiewicz et al. (2017) | No | ASD |
| 3 | Support | - | Jianling Ji et al. (2019) | Yes | - |
| 4 | Support | Large-Scale Exome Sequencing Study Implicates Both Developmental and Functional Changes in the Neurobiology of Autism | Satterstrom FK et al. (2020) | Yes | - |
| 5 | Support | - | Kevin E Glinton et al. (2021) | No | ASD, ADHD |
| 6 | Support | - | Danny Antaki et al. (2022) | Yes | - |
| 7 | Support | - | Zhou X et al. (2022) | Yes | - |
| 8 | Support | - | Fu JM et al. (2022) | Yes | - |
| 9 | Support | - | Ana Blázquez et al. (2025) | Yes | ADHD, DD |
| 10 | Primary | - | Gülsüm Kayhan et al. (2026) | Yes | ADHD |
| 11 | Support | - | Wang, Lulu et al. (2026) | Yes | - |
Rare Variants (42)
| Status | Allele Change | Residue Change | Variant Type | Inheritance Pattern | Parental Transmission | Family Type | PubMed ID | Author, Year |
|---|---|---|---|---|---|---|---|---|
| c.2168G>A | p.Arg723His | missense_variant | De novo | - | - | 35982160 | Fu JM et al. (2022) | |
| c.5709-7C>T | - | splice_region_variant | De novo | - | Simplex | 35982159 | Zhou X et al. (2022) | |
| c.2779G>A | p.Ala927Thr | missense_variant | Unknown | - | - | 42036727 | Wang, Lulu et al. (2026) | |
| c.402G>T | p.Glu134Asp | missense_variant | De novo | - | Simplex | 28263302 | C Yuen RK et al. (2017) | |
| c.8081G>C | p.Arg2694Thr | missense_variant | Unknown | - | - | 33522091 | Kevin E Glinton et al. (2021) | |
| c.6960A>G | p.Ser2320= | synonymous_variant | De novo | - | - | 31981491 | Satterstrom FK et al. (2020) | |
| c.6364A>C | p.Thr2122Pro | missense_variant | De novo | - | Multiplex | 35982159 | Zhou X et al. (2022) | |
| c.1282G>T | p.Glu428Ter | stop_gained | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.8650A>T | p.Lys2884Ter | stop_gained | De novo | - | - | 28942966 | Paweà â Stankiewicz et al. (2017) | |
| c.2203_2204del | p.Arg735fs | frameshift_variant | De novo | - | - | 35654974 | Danny Antaki et al. (2022) | |
| c.2921+1G>C | - | splice_site_variant | Familial | Maternal | - | 33522091 | Kevin E Glinton et al. (2021) | |
| c.4555C>T | p.Arg1519Ter | stop_gained | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.8278G>T | p.Glu2760Ter | stop_gained | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.3610C>T | p.Arg1204Ter | stop_gained | Familial | Maternal | - | 33522091 | Kevin E Glinton et al. (2021) | |
| c.4588C>G | p.Gln1530Glu | missense_variant | Unknown | - | - | 41751633 | Gülsüm Kayhan et al. (2026) | |
| c.3360_3370+1del | - | splice_site_variant | De novo | - | - | 28942966 | Paweà â Stankiewicz et al. (2017) | |
| c.2922-1506_*8577del | - | copy_number_loss | Unknown | - | - | 28942966 | Paweà â Stankiewicz et al. (2017) | |
| c.5770G>A | p.Ala1924Thr | missense_variant | De novo | - | - | 28942966 | Paweà â Stankiewicz et al. (2017) | |
| c.8558T>G | p.Met2853Arg | missense_variant | De novo | - | - | 28942966 | Paweà â Stankiewicz et al. (2017) | |
| c.-121653_2922-3575del | - | copy_number_loss | De novo | - | - | 28942966 | Paweà â Stankiewicz et al. (2017) | |
| c.8210+6_8210+8del | - | splice_region_variant | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.486_512del | p.Glu162_Asp170del | inframe_deletion | De novo | - | Multiplex | 35982159 | Zhou X et al. (2022) | |
| c.7875+3559_7876-2789del | - | copy_number_loss | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.1607_1620del | p.Asp536GlyfsTer5 | frameshift_variant | Unknown | - | - | 33522091 | Kevin E Glinton et al. (2021) | |
| c.8562_8563del | p.Val2855SerfsTer7 | frameshift_variant | De novo | - | - | 40071278 | Ana Blázquez et al. (2025) | |
| c.989del | p.Leu330ArgfsTer28 | frameshift_variant | De novo | - | - | 28942966 | Paweà â Stankiewicz et al. (2017) | |
| c.2860dup | p.Glu954GlyfsTer5 | frameshift_variant | De novo | - | - | 28942966 | Paweà â Stankiewicz et al. (2017) | |
| c.3233_3237del | p.Arg1078MetfsTer13 | frameshift_variant | Unknown | - | - | 33522091 | Kevin E Glinton et al. (2021) | |
| c.255dupC | p.Ser86GlnfsTer43 | frameshift_variant | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.2744del | p.Asn915ThrfsTer36 | frameshift_variant | De novo | - | - | 28942966 | Paweà â Stankiewicz et al. (2017) | |
| c.209dupG | p.Ser71GlnfsTer3 | frameshift_variant | Familial | Maternal | - | 33522091 | Kevin E Glinton et al. (2021) | |
| c.255delC | p.Ser86AlafsTer151 | frameshift_variant | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.6078dup | p.Ala2027CysfsTer2 | frameshift_variant | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.6259+3_6259+4delinsG | p.? | splice_region_variant | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.3085delA | p.Thr1029GlnfsTer27 | frameshift_variant | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.5715_5716delAG | p.Val1906GlufsTer15 | frameshift_variant | De novo | - | Simplex | 30755392 | Jianling Ji et al. (2019) | |
| c.2724_2727del | p.Thr909SerfsTer4 | frameshift_variant | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.5936-1G>A | p.Thr1980GlufsTer25 | splice_site_variant | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.7521_7524dup | p.Leu2509IlefsTer21 | frameshift_variant | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.3210_3221del | p.Asn1071_Glu1074del | inframe_deletion | Familial | Paternal | - | 33522091 | Kevin E Glinton et al. (2021) | |
| c.(7875+1_7876-1)_(8209+1_8210-1)del | - | copy_number_loss | De novo | - | Simplex | 33522091 | Kevin E Glinton et al. (2021) | |
| c.5216_5217del | p.Val1739GlyfsTer96 | frameshift_variant | Unknown | Not maternal | - | 28942966 | Paweà â Stankiewicz et al. (2017) |
Common Variants
No common variants reported.
SFARI Gene score
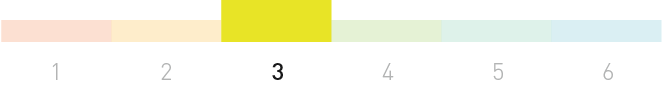
Suggestive Evidence
criteria met
See SFARI Gene'scoring criteriaThe literature is replete with relatively small studies of candidate genes, using either common or rare variant approaches, which do not reach the criteria set out for categories 1 and 2. Genes that had two such lines of supporting evidence were placed in category 3, and those with one line of evidence were placed in category 4. Some additional lines of "accessory evidence" (indicated as "acc" in the score cards) could also boost a gene from category 4 to 3.
4/1/2026
Initial score established: 3
Krishnan Probability Score
Score 0.60900141696863
Ranking 270/25841 scored genes
[Show Scoring Methodology]
ExAC Score
Score 0.99999999999524
Ranking 48/18225 scored genes
[Show Scoring Methodology]
Sanders TADA Score
Score 0.9499712828023
Ranking 18306/18665 scored genes
[Show Scoring Methodology]
Zhang D Score
Score 0.57711876256878
Ranking 144/20870 scored genes
[Show Scoring Methodology]